
Introduction
In recent decades, invasive fungal infections have increased significantly, reaching an unacceptable global annual incidence rate of 6.5 million cases with 3.8 million deaths, ~66% (2.5 million deaths) of which are directly attributable to these infections [ 1 ]. Invasive candidiasis is a serious infection caused by various species of Candida. It is the most common fungal disease found in hospitals in high-income countries. Global prevalence of this infection ranges from 250,000 to approximately 700,000 cases per year, with an incidence rate of 2-14 cases per 100,000 individuals. The mortality rates associated with this disease are 40-55% [ 2 ]. Candida infections are among the top 10 pathogens commonly identified in intensive care units or immunocompromised patients. They account for as much as 10% of bloodstream infections acquired in hospitals, outpacing several prevalent bacterial species, including Pseudomonas aeruginosa [ 3 ]. However, Candida species can also cause superficial infections [ 4 ]. Although Candidaalbicans remains the most commonly encountered pathogen in clinical samples, an epidemiological shift towards non-albicans Candida species has been repeatedly reported in many geographic areas, which is of growing concern worldwide [ 3 , 5 - 7 ].
The growing public health threat posed by new and old Candida species, and other fungal agents, has also been recognized by the World Health Organization, which recently published the first fungal priority pathogens list to raise awareness of fungal infections and support research on antifungal resistance [ 8 ]. This list includes 19 pathogens, most of which are intrinsically resistant to commonly used antifungal agents or capable of rapidly developing resistance upon repeated exposure to the drug [ 9 ].
Azoles, echinocandins, and polyenes are classes of antifungal drugs commonly used to treat Candida infections, with azoles being the most frequently used for treatment and prevention [ 10 ]. Unfortunately, in recent years, the overuse of azoles for long-term prophylaxis or therapy has led to azole resistance as a growing problem, thus increasing the difficulty of treatment [ 11 , 12 ]. Candida albicans holds key genes and molecular mechanisms related to azole resistance [ 11 ], including the increased expression of drug efflux pumps that are encoded by the CDR1, CDR2, and MDR1 genes, altered expression or mutations in the ERG11 gene encoding lanosterol 14-α-demethylase, loss of heterozygosity at certain loci, particularly TAC1 and MRR1, and mutations in zinc cluster transcription factors, such as TAC1, MRR1, and UPC2, which work independently or together to create varying degrees of azole resistance in C. albicans (Figure 1) [ 11 , 13 ]. The UPC2 is a zinc (II)-Cys (6) transcription factor that plays a role in sterol biosynthesis and azole resistance. Initially recognized as a homolog of the S. cerevisiae (ScUPC2) gene, the UPC2 gene in C. albicans has been shown to enhance the expression of ergosterol biosynthesis genes ERG2 and ERG11 when exposed to fluconazole [ 11 ]. Overexpression of ERG11 has been shown to reduce azole susceptibility by increasing the production of the azole target 14α-lanosterol demethylase. Additionally, UPC2 controls sterol uptake without oxygen and regulates other environmental adaptations, including anaerobic conditions, contributing to azole resistance [ 14 ]. This review will explore the structure and function of the UPC2 gene, as well as its involvement in azole resistance, addressing the existing knowledge gaps in this area.
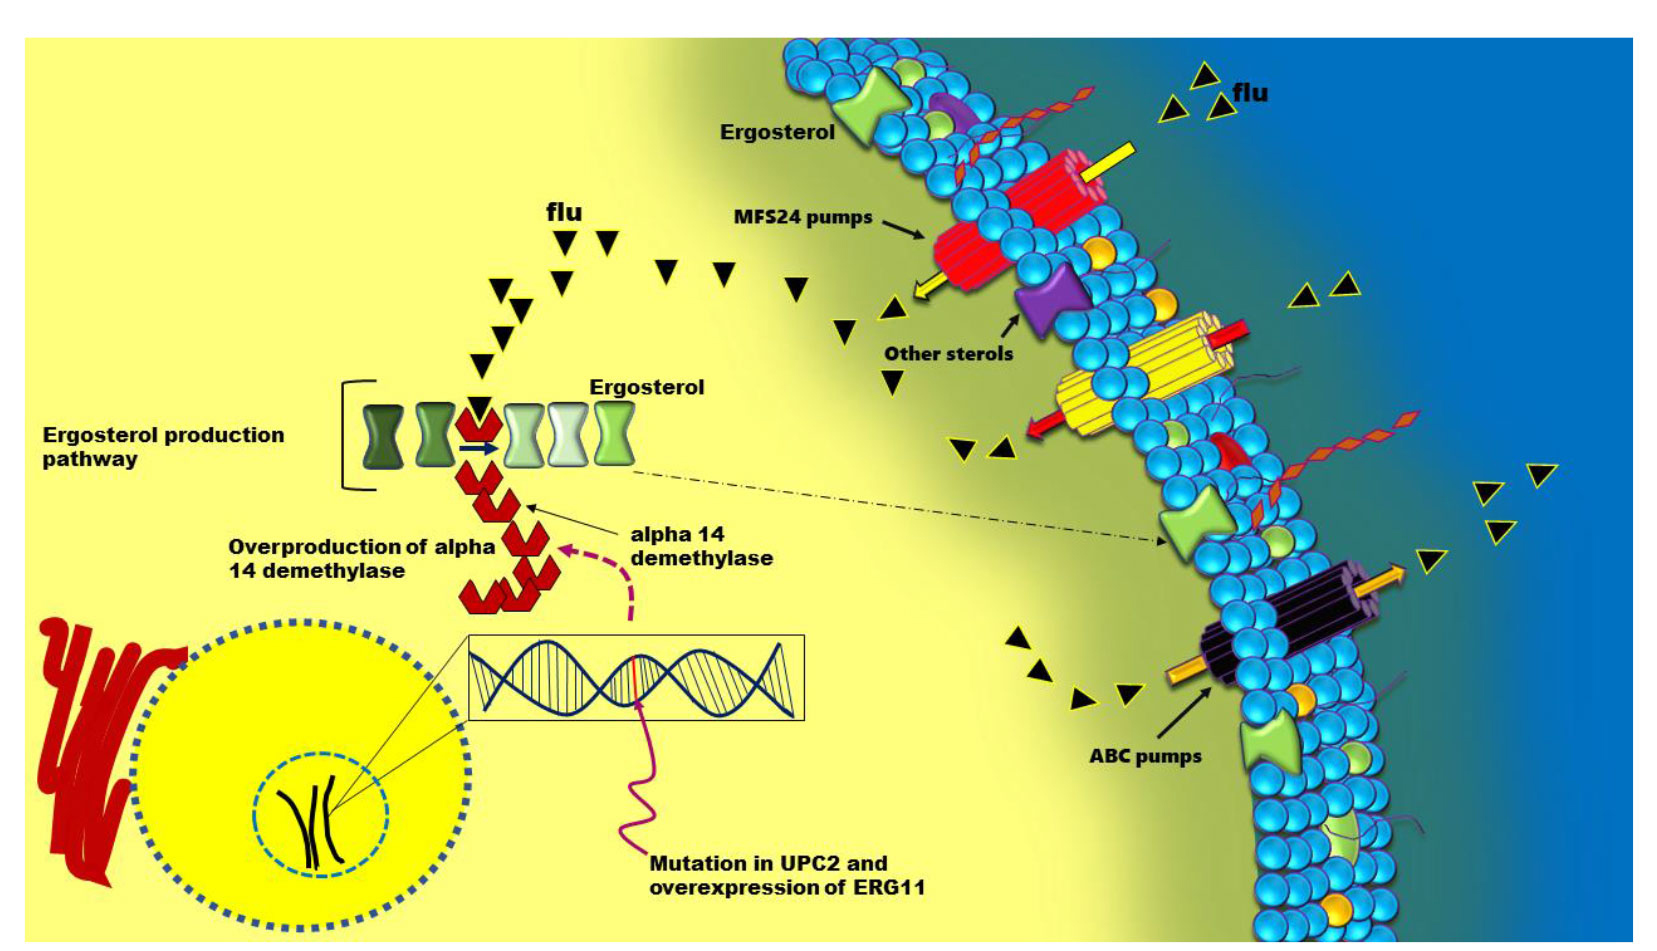
Figure 1. Graphical representation summarizing the reduced susceptibility to azoles of Candida spp. due to DNA changes occurring in the UPC2 gene. Specific mutations of this gene result in the transcriptional upregulation of the ERG11 gene leading to overproduction of the enzyme lanosterol 14-α-demethylase and, ultimately, to fluconazole resistance.
Data collection
The current mini-review was conducted through online literature searches of peer-reviewed articles published between January 1, 1999, and April 21, 2024, and indexed in the following three authoritative databases: Scopus, PubMed, and Web of Science. The inclusion and exclusion criteria in this study were as follows:
Inclusion criteria:
Studies on C. albicans: Articles focusing on the biology, genetics, and drug resistance mechanisms of C. albicans, specifically concerning the UPC2 gene.
Azole resistance studies: Research that investigates resistance mechanisms to azole antifungal drugs, including mutations, regulatory pathways, or gene expression analysis.
Peer-reviewed publications: Articles published in peer-reviewed journals to ensure the reliability and scientific rigor of the data.
English language: Studies published in English to maintain consistency in interpretation.
Time frame: Articles published between January 1, 1999, and April 21, 2024, as defined in the manuscript.
Keywords: Studies using terms, such as “UPC2 gene”, “C. albicans”, “azole resistance”, and “resistance mechanism.”
Exclusion criteria:
Non-English publications: Studies published in languages other than English.
Non-peer-reviewed sources: Articles from non-peer-reviewed sources, including preprints or gray literature.
Non-Candida species studies: Research focusing on organisms other than C. albicans (e.g., Aspergillus or non-albicans Candida).
Unrelated topics: Studies that did not address the UPC2 gene, azole resistance, or related genetic and molecular mechanisms.
Inadequate data: Articles lacking sufficient experimental data or those that are purely theoretical without substantive evidence supporting their conclusions.
Structure of UPC2 gene
According to the Candida genome database (www.Candidagenome.org), in C. albicans, the 2,139 bp long-UPC2 gene (orf19.391) is located on chromosome 1 and encodes a zinc-cluster transcription factor of 712 amino acids. The gene has orthologues in other pathogenic Candida species (C. auris, C. dubliniensis, and C. parapsilosis) and other fungi, including Saccharomyces cerevisiae where an additional paralogous gene (ECM22) is also present (www.yeastgenome.org) [ 15 - 17 ].
This family of transcriptional regulators, with over 80 members, is a highly conserved fungal-specific family of transcription factors with a Zn(2)-Cys(6) binuclear cluster domain [ 18 ].Sequence analysis of the UPC2 gene in C. albicans has revealed two key domains, namely an anchoring transmembrane domain and a region associated with transcription factors that include several nuclear localization signals and a fungal Zn(2)-Cys(6) binuclear cluster domain [ 18 ]. The UPC2 regulates the expression of ERG11 and most of the genes in the ergosterol biosynthesis pathway on some level (Figure 2) [ 19 ]. Ergosterol is a fundamental component of the fungal cell membrane, and, therefore, its biosynthetic pathway is the primary target for most antifungal compounds currently used to treat severe fungal infections (allylamines, azoles, and morpholines) [ 20 ].
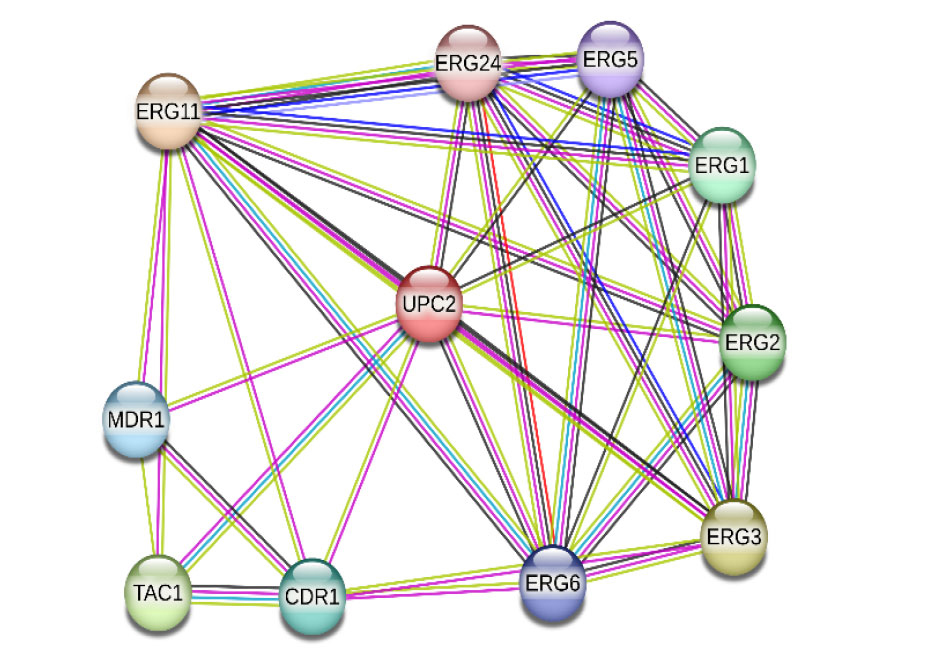
Figure 2. A protein-protein communication network between UPC2 and other effector gene products in C. albicans. The interaction network was constructed using the STRING database version 11.0 (https://string-db.org). The confidence score threshold was set to be more than 0.7, while the species was "C. albicans" (Cytoscape version 3.7.1, www.cytoscape.org). The edges are categorized based on the source of interaction data: known interactions are derived from curated databases (represented by blue lines) and experimentally determined interactions (pink lines), while predicted interactions are indicated by green lines (gene neighborhood), red lines (gene fusions), and blue lines (gene co-occurrence). Additionally, other sources of associations include text mining (yellow lines), co-expression (black lines), and protein homology (light blue lines).
Azole exposure can lead to overexpression of the UPC2 gene, which can adequately compensate for the inhibition of target enzymes [ 19 ]. While UPC2 disruption results in reduced accumulation of exogenous sterols and hyper-susceptibility to fluconazole [ 21 ]. Previous studies have indicated that UPC2 may also trigger MDR1 expression, playing a minor role in the regulation of multidrug efflux pumps and MDR1-mediated drug resistance. However, MRR1 is a more significant regulator of this efflux pump [ 22 ].
Zinc cluster family of transcription factors, which includes TAC1p, MRR1p, and UPC2p proteins, is exclusive to fungi. These transcription factors are crucial for helping C. albicans cells to adapt to drug pressure and other general stresses [ 23 , 24 ]. The UPC2 gene in C. albicans encodes a 712 amino acid protein essential in sterol biosynthesis regulation and drug resistance [ 25 ]. The structure of the UPC2 protein (Figure 3) includes different domains with specific structural and functional features, essential for successful interaction with cellular targets. For example, the amino-terminal (N-terminal) DNA-binding domain, characterized by a conserved Zn (II)2-Cys6 zinc finger motif, is essential for the response to sterol levels in the cell [ 17 , 26 ]. While the carboxyl-terminal (C-terminal) regulatory domain is fundamental for responding to intracellular sterol levels and their regulation [ 27 , 28 ]. In addition, the UPC2 protein also contains a C-terminal ligand-binding domain (LBD) consisting of 11 α-helices and connecting loops, folded to form a closed clamp that creates a deep hydrophobic pocket in the core of the protein, providing enough space for binding sterol molecules [ 28 ]. The C-terminal LBD of UPC2 adopts a novel α-helical fold involved in ligand binding, particularly sterols, like ergosterol [ 28 ].
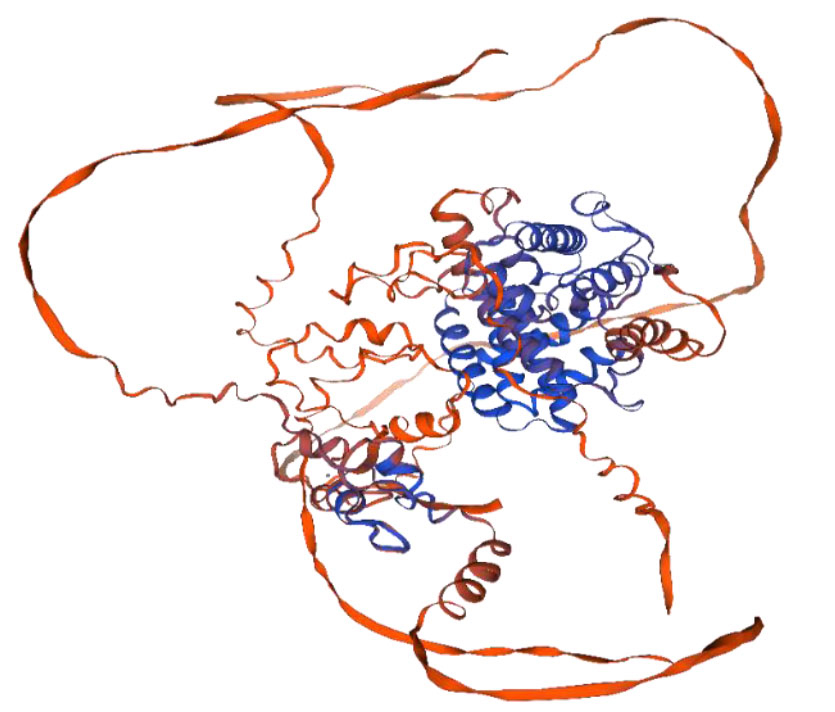
Figure 3. A 3D homology-based model of UPC2 protein predicted using the Swiss Model tool on the ExPASy server. The ribbon model shows the protein backbone with a color gradient from blue to orange and red. The blue regions represent the structured core or DNA-binding domain that is essential for protein function, while the orange to red regions represent more flexible regions that may facilitate interactions with other molecules or allow the protein to change its shape according to functional-regulatory needs. Amino acids at positions 54-81 (Sequence: CSTCKKRRVKCDEQRPVCGNCTKLKLDC) are the DNA binding region.
Gain-of-function (GOF) mutations in UPC2 can lead to increased expression of the ERG11 gene encoding for the lanosterol 14α-demethylase, an essential enzyme of the ergosterol biosynthetic pathway [ 19 , 29 ]. This protein is the target of the azole drugs and its inhibition results in a depletion of ergosterol, accumulation of toxic sterols, and inhibition of fungal growth [ 30 , 31 ]. Overexpression of the ERG11 gene has been found to lead to higher levels of cellular ergosterol and reduced susceptibility to azole drugs by enhancing the production of the enzyme that targets azoles [ 11 ].
Sequence analysis of UPC2 alleles of fluconazole-resistant isolates showed that specific single-nucleotide polymorphisms (SNPs) generate dominant GOF mutations, such as the UPC2G648D, UPC2Y642F or UPC2A643V amino acid substitutions. This leads to a constant upregulation of the ERG11 promoter, which in turn, grants fluconazole resistance to clinical isolates of C. albicans [ 29 ]. However, the exact mechanism underlying UPC2-mediated gene upregulation still remains unknown [ 29 , 32 ]. Types of mutations of the UPC2 gene investigated in previous studies are listed in Table 1.
| Author (year) Reference | Strains | Mutation of UPC2 | Function |
|---|---|---|---|
| Nico Dunkel (2008) [ 21 ] | S2 (Fluconazole-resistant isolate from the patient)- Candida albicans | G648D | Elevated levels of ERG11 expression and imparted fluconazole resistance |
| Clemens J. Heilmann (2009) [ 32 ] | Isolate 5052 (Fluconazole-resistant isolate from the patient)- C. albicans | G1927A | This resulted in an exchange of alanine for threonine at position 643 (A643T) in the encoded protein and increased ERG11 and UPC2 expression |
| Florent Morio (2013) [ 39 ] | CAAL28: HIV1 patient (C. albicans) | I142Sh3, A451Vh | Not mentioned |
| CAAL37: Rheumatoid arthritis patient (C. albicans) | R68Kh, I142Sh, S190Nh, S228Nh | Not mentioned | |
| CAAL 61: HIV patient (C. albicans) | I142S, G648S | GOF mutation | |
| CAAL 67: HIV patient (C. albicans) | I142Sh | Not mentioned | |
| CAAL74: SCID2 patient (C. albicans) | R68Kh, I142S, S228Nh, T273Ah, G648Sh, K684Eh | GOF mutation, T273A and K684E: Elevated levels of ERG11 expression and imparts fluconazole resistance | |
| CAAL 75: HIV patient (C. albicans) | R68Kh, I142Sh, S228Nh, K684Eh, T273Ah | T273A and K684E: Elevated levels of ERG11 expression and imparts fluconazole resistance | |
| Stephanie A. Flowers (2012) [ 29 ] | 6 fluconazole-resistant clinical ERG11-overexpressing isolates | G648D | Elevated levels of ERG11 expression and imparted fluconazole resistance |
| 9 fluconazole-resistant clinical ERG11-overexpressing isolates | G648S | Elevated levels of ERG11 expression and imparted fluconazole resistance | |
| 1 fluconazole-resistant clinical ERG11-overexpressing isolates | A643T | Elevated levels of ERG11 expression and imparted fluconazole resistance | |
| 2 fluconazole-resistant clinical ERG11-overexpressing isolates | A643V | Elevated levels of ERG11 expression and imparted fluconazole resistance | |
| 2 fluconazole-resistant clinical ERG11-overexpressing isolates | A646V | Elevated levels of ERG11 expression and imparted fluconazole resistance | |
| 2 fluconazole-resistant clinical ERG11-overexpressing isolates | Y642F | Elevated levels of ERG11 expression and imparted fluconazole resistance | |
| 3 fluconazole-resistant clinical ERG11-overexpressing isolates | W478C | Elevated levels of ERG11 expression and imparted fluconazole resistance | |
| 2 fluconazole-resistant clinical ERG11-overexpressing isolates | G304R | This mutation does not result in the gain of function | |
| Samantha J. Hoot (2011) [ 36 ] | 17 azole-resistant strains of C. albicans | A643V | In the A643V clinical isolates and reconstructed strains, there were increased levels of azole susceptibility, ergosterol, and expression of ERG genes |
| Christina Popp (2017) [ 37 ] | F5 (fluconazole-resistant clinical isolate, C. albicans) | G648S | ERG11 overexpression and increased drug resistance |
| G1942A | Not mentioned | ||
| TW17 (fluconazole-resistant clinical isolate, C. albicans) | A643V | ERG11 overexpression and increased drug resistance | |
| Roy A. Khalaf (2021) [ 41 ] | CA77 (clinical isolate, C. albicans) | I142S | A recognized mutation that has not been previously associated with antifungal resistance |
| Emilie Sitterlé (2020) [ 40 ] | 151 unrelated C. albicans strains susceptible to fluconazole and caspofungin | L25Fh, K26E, T41Nh, R68K, I142S, T144Ih, S190N, A221P, S228N, N250Sh, T273A, G321Sh, L342Vh, V507Ih, L635Wh | No conferred increases in azole MICs |
| 1: Human immunodeficiency virus; 2: Severe combined immunodeficiency; h: heterozygous (mutation in a single allele); MIC: minimum inhibitory concentration | |||
Discussion
The most frequently prescribed antifungal medications for infections caused by C. albicans are azoles, which work by inhibiting the enzyme 14-α-sterol demethylase, encoded by the ERG11 gene [ 33 ]. Nucleotide changes in this gene can generate missense mutations affecting the azole-binding domain of the protein, thus conferring resistance or reduced susceptibility to these drugs. Moreover, overexpression of ERG11 leads to the increased production of the target enzyme, contributing to the evolution of azole-resistant isolates. An important key regulator of the expression of the ERG11 gene is the zinc cluster protein UPC2 whose inhibition leads to hypersensitivity to azoles and a reduced uptake of alternative sterols into C. albicans cell membrane. Recently, the critical role of UPC2 in C. auris was highlighted by the regulation of the activation of the MRR1/MDR1 pathway and the ergosterol biosynthesis pathway [ 34 , 35 ]. Exposure of Candida to azole leads to GOF and overexpression of UPC2, which inhibits the target enzymes and results in resistance to azoles [ 21 ]. McPherson et al. and Silver et al. introduced the UPC2p as a key regulator of ergosterol metabolism in C. albicans [ 17 , 18 ] who first demonstrated that in the absence of UPC2, the azole-inducible expression of ERG2, ERG7, ERG11, and ERG25 genes was decreased.
Researchers have identified numerous substitutions in the UPC2 gene linked to the development of azole resistance. Previous studies have mainly focused on the mutation related to the I142S amino acid substitution in the UPC2 protein. However, it does not appear to be linked to azole resistance since it was also detected in azole-susceptible C. albicans isolates [ 25 ].
The A643V substitution in the UPC2 is another mutation that increases fluconazole resistance in clinical Candida isolates [ 36 ]. This mutation affects the C-terminal regulatory domain of UPC2 disrupting its function and upregulating the ERG11 expression in resistant isolates [ 36 ].
In a study conducted by Flower et al. in 2012 [ 29 ], eight distinct mutations of the UPC2 gene (G648D, G648S, A643T, A643V, Y642F, G304R, A646V, and W478C) were identified in 29 out of 47 isolates of C. albicans. Notably, seven of these mutations (87.5%) led to higher expression levels of the ERG11 gene and increased cellular ergosterol, resulting in decreased sensitivity to fluconazole when compared to wild-type strains. Genes affected by these variations were found to be involved in ergosterol biosynthesis, oxidoreductase activity, and the major efflux pump encoded by the MDR1 gene [ 29 ]. The UPC2 GOF mutations are common in clinical isolates, but not necessarily in all isolates less susceptible to azoles [ 37 ]. For example, the highest expression of the ERG11 gene is associated with the amino acid substitution G648D and, therefore, different effects might be observed in the mutant strains during antifungal susceptibility testing, depending on the type of substitution and the antifungal drug used [ 38 ]. Previous studies have shown that the strains expressing the G304R mutant allele did not have any decrease in antifungal susceptibility. In contrast, an increase in MIC values for fluconazole and terbinafine was observed in the strains expressing G648D, G648S, A643T, A643V, Y642F, W478C, and A646V mutations [ 29 ].
In another study, Popp et al. in 2017 [ 37 ] identified three UPC2 GOF mutations, namely G648S, G1942, and A643V, in two fluconazole-resistant clinical C. albicans isolates, F5 and TW17. They found these mutations caused a significant fitness defect when isolates were grown for 24 h in a yeast extract-peptone-dextrose medium. Furthermore, the same authors noted that the fitness costs of drug resistance are also likely to depend on the individual host [ 37 ].
In line with previous studies [ 39 , 40 ], Khalaf et al. [ 41 ] utilized whole genome sequencing to identify 19-point mutations across eight genes (ERG11, ERG24, ERG251, UPC2, CDR1, MRR2|, FKS1, and GLS1) in the azole-resistant C. albicans strain known as CA77, which was isolated from a stool sample. Other UPC2 mutations were identified by large-scale genome sequencing performed by Sitterlé et al. [ 40 ], and two substitutions, D654N and G657D, were reported as new putative mutations involved in antifungal resistance.
Given the increasing resistance of Candida species to common antifungal agents, especially azoles [ 42 ], and also considering the high plasticity of Candida genomes [ 43 , 44 ], it is important to identify rapid DNA mutations that lead to drug resistance under different environmental conditions. Based on our review of various studies from 1997 to 2024, most of the mutations identified in the UPC2 gene so far result in overexpression of the ERG11 gene, although the role of some of them is still unclear.
Conclusion
Overall, the UPC2 gene plays a key role in the emergence of Candida-resistant phenotypes to azole antifungal drugs. With scientific advances in the use of new DNA sequencing techniques, different resistance pathways are expected to be discovered in the future. Knowledge of the molecular mechanisms underlying antifungal resistance and point mutations in genes involved in this phenomenon is important to guide the development of novel fungal therapeutics and diagnostics.
Acknowledgements
None to declare.
Authors’ contribution
A. H., A. H. M., and I. H. conceived and designed the analysis. A. H., M. G. H., M. A., and F. K. collected the data. S. S. B., A. H., M. E., and A. B., contributed data or analysis tools. S. S. B., A. B., Z. F., and M. M. performed the analysis. A. H., A. H. M., F. K., M. E., M. A., M. M., and I. H. wrote the article. I. H., M. A. reviewed and edited the manuscript. All authors have reviewed and approved the final version of the article before submission.
Conflicts of interest
The authors declare no commercial or financial relationships that could be construed as a potential conflict of interest.
Financial disclosure
This research received no specific grant from any funding agency in the public, commercial, or not-for-profit sectors.
References
- Denning DW. Global incidence and mortality of severe fungal disease. Lancet Infect Dis. 2024; 24(7):e428-e438.
- Soriano A, Honore PM, Puerta-Alcalde P, Garcia-Vidal C, Pagotto A, Gonçalves-Bradley DC, Verweij PE. Invasive candidiasis: current clinical challenges and unmet needs in adult populations. J Antimicrob Chemother. 2023; 78(7):1569-1585.
- Lass-Flörl C, Kanj SS, Govender NP, Thompson III GR, Ostrosky-Zeichner L, Govrins MA. Invasive candidiasis. Nat Rev Dis Primers. 2024; 10(1):20.
- Kaushik N, Pujalte GG, Reese ST. Superficial Fungal Infections. Prim Care. 2015; 42(4):501-16.
- Twenty years of the SENTRY antifungal surveillance program: results for Candida species from 1997–2016. Open forum infectious diseases. 2019; 6(Suppl-1):S79-S94.
- Arastehfar A, Gabaldón T, Garcia-Rubio R, Jenks JD, Hoenigl M, Salzer HJ, et al. Drug-resistant fungi: an emerging challenge threatening our limited antifungal armamentarium. Antibiotics. 2020; 9(12):877.
- Dougue AN, El‐Kholy MA, Giuffrè L, Galeano G, D′ Aleo F, Kountchou CL, et al. Multilocus sequence typing (MLST) analysis reveals many novel genotypes and a high level of genetic diversity in Candida tropicalis isolates from Italy and Africa. Mycoses. 2022; 65(11):989-1000.
- Organization WH. WHO fungal priority pathogens list to guide research, development and public health action: World Health Organization; 2022.
- van Rhijn N, Arikan-Akdagli S, Beardsley J, Bongomin F, Chakrabarti A, Chen SC, et al. Beyond bacteria: the growing threat of antifungal resistance. The Lancet. 2024; 404(10457):1017-1018.
- Rabaan AA, Sulaiman T, Al-Ahmed SH, Buhaliqah ZA, Buhaliqah AA, AlYuosof B, et al. Potential Strategies to Control the Risk of Antifungal Resistance in Humans: A Comprehensive Review. Antibiotics. 2023; 12(3):608.
- Nishimoto AT, Sharma C, Rogers PD. Molecular and genetic basis of azole antifungal resistance in the opportunistic pathogenic fungus Candida albicans. J Antimicrob Chemother. 2020; 75(2):257-70. DOI
- Nishimoto AT, Sharma C, Rogers PD. Candida albicans heat shock proteins and Hsps-associated signaling pathways as potential antifungal targets. Front Cell Infect Microbiol. 2017; 7:520.
- Xiang M-J, Liu J-Y, Ni P-H, Wang S, Shi C, Wei B, et al. Erg11 mutations associated with azole resistance in clinical isolates of Candida albicans. FEMS Yeast Res. 2013; 13(4):386-93.
- Joshua IM, Höfken T. From Lipid Homeostasis to Differentiation: Old and New Functions of the Zinc Cluster Proteins Ecm22, Upc2, Sut1 and Sut2. Int J Mol Sci. 2017; 18(4):772.
- Candida Genome database. 2024.
- Davari A, Haghani I, Hassanmoghadam F, Nabili M, Shokohi T, Hedayati MT, et al. Echinocandin resistance in Candida parapsilosis sensu stricto: Role of alterations in CHS3, FKS1 and Rho gene expression. J Glob Antimicrob Resist. 2020; 22:685-8.
- MacPherson S, Akache B, Weber S, De Deken X, Raymond M, Turcotte B. Candida albicans zinc cluster protein Upc2p confers resistance to antifungal drugs and is an activator of ergosterol biosynthetic genes. Antimicrob Agents Chemother. 2005; 49(5):1745-1752.
- Silver Peter M, Oliver Brian G, White Theodore C. Role of Candida albicans Transcription Factor Upc2p in Drug Resistance and Sterol Metabolism. Eukaryotic Cell. 2004; 3(6):1391-7.
- Czajka KM, Venkataraman K, Brabant-Kirwan D, Santi SA, Verschoor C, Appanna VD, et al. Molecular Mechanisms Associated with Antifungal Resistance in Pathogenic Candida Species. Cells. 2023; 12(22):2655.
- Rodrigues Marcio L. The Multifunctional Fungal Ergosterol. mBio. 2018; 9(5):e01755-18.
- Dunkel N, Liu TT, Barker KS, Homayouni R, Morschhäuser J, Rogers PD. A gain-of-function mutation in the transcription factor Upc2p causes upregulation of ergosterol biosynthesis genes and increased fluconazole resistance in a clinical Candida albicans isolate. Eukaryot Cell. 2008; 7(7):1180-1190.
- Schubert S, Barker KS, Znaidi S, Schneider S, Dierolf F, Dunkel N, et al. Regulation of efflux pump expression and drug resistance by the transcription factors Mrr1, Upc2, and Cap1 in Candida albicans. Antimicrob Agents Chemother. 2011; 55(5):2212-23.
- Znaidi S, Weber S, Al-Abdin OZ, Bomme P, Saidane S, Drouin S, et al. Genomewide location analysis of Candida albicans Upc2p, a regulator of sterol metabolism and azole drug resistance. Eukaryot Cell. 2008; 7(5):836-47.
- Vasicek Erin M, Berkow Elizabeth L, Flowers Stephanie A, Barker Katherine S, Rogers PD. UPC2 Is Universally Essential for Azole Antifungal Resistance in Candida albicans. Eukaryotic Cell. 2014; 13(7):933-46.
- Fattouh N, Hdayed D, Hijazi A, Tokajian S, Khalaf RA. UPC2 mutations and development of azole resistance in Candida albicans hospital isolates from Lebanon. J Glob Antimicrob Resist. 2024; 38:341-348.
- Kakade P, Mahadik K, Balaji KN, Sanyal K, Nagaraja V. Two negative regulators of biofilm development exhibit functional divergence in conferring virulence potential to Candida albicans. FEMS Yeast Res. 2018; 19(2)
- Ha S, Tong J, Yang H, Youn HS, Eom SH, Im YJ. Crystallization and preliminary X-ray crystallographic analysis of sterol transcription factor Upc2 from Saccharomyces cerevisiae. Acta Crystallogr Sect F Struct Biol Cryst Commun. 2013; 69(Pt 2):147-152.
- Yang H, Tong J, Lee CW, Ha S, Eom SH, Im YJ. Structural mechanism of ergosterol regulation by fungal sterol transcription factor Upc2. Nature Communications. 2015; 6(1):6129.
- Flowers SA, Barker KS, Berkow EL, Toner G, Chadwick SG, Gygax SE, et al. Gain-of-function mutations in UPC2 are a frequent cause of ERG11 upregulation in azole-resistant clinical isolates of Candida albicans. Eukaryot Cell. 2012; 11(10):1289-1299.
- Rosam K, Monk BC, Lackner M. Sterol 14α-Demethylase Ligand-Binding Pocket-Mediated Acquired and Intrinsic Azole Resistance in Fungal Pathogens. Journal of fungi (Basel, Switzerland). 2020; 7(1)
- Stenkiewicz-Witeska JS, Ene IV. Azole potentiation in Candida species. PLoS pathogens. 2023; 19(8):e1011583.
- Heilmann CJ, Schneider S, Barker KS, Rogers PD, Morschhäuser J. An A643T mutation in the transcription factor Upc2p causes constitutive ERG11 upregulation and increased fluconazole resistance in Candida albicans. Antimicrob Agents Chemother. 2010; 54(1):353-359.
- Whaley SG, Berkow EL, Rybak JM, Nishimoto AT, Barker KS, Rogers PD. Azole antifungal resistance in Candida albicans and emerging non-albicans Candida species. Front microbiol. 2017; 7:231851.
- Khojasteh S, Jafarzdeh J, Hosseini SA, Haghani I, Turki H, Aghaei Gharehbolagh S, et al. Candida auris and COVID-19: A health threatening combination. Curr Med Mycol. 2022; 8(3):44-50.
- Li J, Aubry L, Brandalise D, Coste AT, Sanglard D, Lamoth F. Upc2-mediated mechanisms of azole resistance in Candida auris. Microbiol Spectr. 2024; 12(2):e03526-23.
- Hoot SJ, Smith AR, Brown RP, White TC. An A643V amino acid substitution in Upc2p contributes to azole resistance in well-characterized clinical isolates of Candida albicans. Antimicrob Agents Chemother. 2011; 55(2):940-942.
- Popp C, Hampe IAI, Hertlein T, Ohlsen K, Rogers PD, Morschhäuser J. Competitive Fitness of Fluconazole-Resistant Clinical Candida albicans Strains. Antimicrob Agents Chemother. 2017; 61(7):e00584-17.
- Sasse C, Dunkel N, Schäfer T, Schneider S, Dierolf F, Ohlsen K, Morschhäuser J. The stepwise acquisition of fluconazole resistance mutations causes a gradual loss of fitness in C andida albicans. Mol Microbiol. 2012; 86(3):539-556.
- Morio F, Pagniez F, Besse M, Gay-Andrieu F, Miegeville M, Le Pape P. Deciphering azole resistance mechanisms with a focus on transcription factor-encoding genes TAC1, MRR1 and UPC2 in a set of fluconazole-resistant clinical isolates of Candida albicans. Int J Antimicrob Agents. 2013; 42(5):410-415.
- Sitterlé E, Coste AT, Obadia T, Maufrais C, Chauvel M, Sertour N, et al. Large-scale genome mining allows identification of neutral polymorphisms and novel resistance mutations in genes involved in Candida albicans resistance to azoles and echinocandins. J Antimicrob Chemother. 2020; 75(4):835-848.
- Khalaf RA, Fattouh N, Medvecky M, Hrabak J. Whole genome sequencing of a clinical drug resistant Candida albicans isolate reveals known and novel mutations in genes involved in resistance acquisition mechanisms. J Med Microbiol. 2021; 70(4)
- Pristov K, Ghannoum M, Fidsa Resistance of Candida to azoles and echinocandins worldwide. Clin Microbiol Infect. 2019; 25DOI
- Selmecki A, Forche A, Berman J. Genomic plasticity of the human fungal pathogen Candida albicans. Eukaryotic cell. 2010; 9(7):991-1008.
- O’Brien CE, Oliveira-Pacheco J, Ó Cinnéide E, Haase MA, Hittinger CT, Rogers TR, et al. Population genomics of the pathogenic yeast Candida tropicalis identifies hybrid isolates in environmental samples. PLoS pathogens. 2021; 17(3):e1009138.


